The review, published as an open access article on 25 September 2026, proposes an integrated framework that combines resistant genotypes with rapid drying to safe moisture limits and improved storage systems tailored to the people who actually handle the crop.
The authors frame their argument around three recurring themes that they say previous work has blurred. First, genotypic resistance alone is not sufficient to reduce aflatoxin contamination, because its expression depends tightly on storage conditions, particularly moisture content and water activity, which regulate fungal growth and toxin biosynthesis. Second, inconsistencies in reported resistance often stem from a failure to distinguish between pre-harvest and post-harvest contamination, which can lead researchers to misjudge how a genotype will actually perform. Third, emerging biochemical evidence indicates that resistance is not the product of a single gene but of coordinated interactions among physical barriers such as seed coat integrity, antifungal metabolites including phenolics and oxylipins, and host-pathogen signaling pathways.
The biology behind the problem is well characterized. Aflatoxins are highly toxic secondary metabolites produced primarily by fungi in the genus Aspergillus, with the major naturally occurring forms designated AFB1, AFB2, AFG1 and AFG2. AFB1 is the most prevalent and the most toxic, and the International Agency for Research on Cancer has classified it as a Group 1 hepatotoxic and hepatocarcinogenic compound. Biosynthesis proceeds through a polyketide pathway from acetyl-CoA and malonyl-CoA precursors, involving more than 18 enzymatic reactions and more than 25 to 30 clustered genes located within approximately 70 to 75 kilobases of fungal genomic DNA. After ingestion of contaminated food, AFB1 is rapidly absorbed and metabolized mainly in the liver by the enzymes CYP1A2 and CYP3A4 into a reactive epoxide that can bind to DNA, RNA and proteins, leading to mutations, hepatocellular damage and liver cancer.
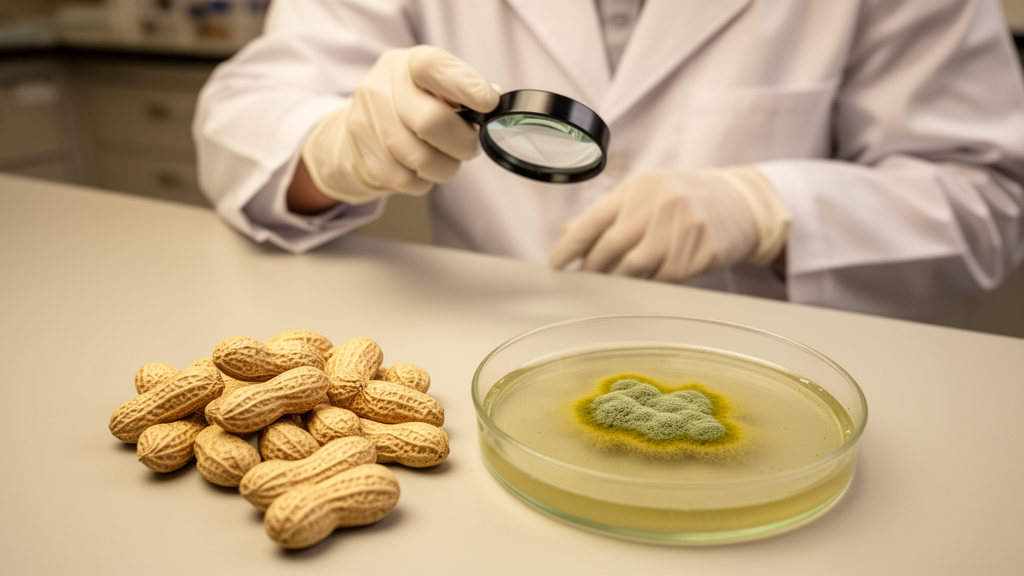
Environmental conditions and fungal genetic variation strongly influence how much toxin is produced. High temperatures between 25 and 35 degrees Celsius, water activity above 0.85, moisture content above 13 percent, drought stress and oxidative stress all promote fungal growth and toxin synthesis, the review reports. Colonization is further shaped by the genetic variability of fungal strains, the nutrient composition of the seed and the presence of competing microorganisms. Some Aspergillus genotypes are incapable of aflatoxin biosynthesis altogether because of deletions or mutations in the biosynthetic gene cluster, a fact that underpins biological control approaches using atoxigenic strains. Fungal spores reach developing pods through damaged shells or via soil contact in the field, while in storage the fungi can spread on improperly dried peanuts or through insect-mediated movement.
Among the crops examined, peanuts stand out for their susceptibility. Multiple studies indicate that peanuts tend to accumulate higher levels of aflatoxins than maize and other staples, and surveys of peanut samples have found levels exceeding strict European regulatory limits, suggesting generally high contamination in both field and storage settings. Regulations for safe aflatoxin levels vary globally but often fall within 2 to 20 micrograms per kilogram for total aflatoxins in grains. The review notes that contamination in stored peanuts can rise markedly over time, with measured levels increasing from low values early in storage to high concentrations in traditional storage conditions, reaching up to approximately 27.6 parts per billion in some samples, a level that can exceed safety limits and compromise product quality.
Genotypic variation is real and measurable. Laboratory studies under controlled storage conditions and artificial inoculation have shown that peanut genotypes respond differently to the emergence and growth of aflatoxigenic fungi, and that genotypes with thinner seed coats or lower levels of antifungal compounds tend to accumulate higher toxin levels. Tengey and colleagues identified two genotypes, ICGV-03401 and L027B, with notably lower aflatoxin accumulation, while Yue and colleagues reported two accessions, Zh.h0551 and Zh.h2150, with reduced aflatoxin B1 and B2 levels and associated SNP markers, providing a genomic basis for resistance breeding. Resistance is a complex quantitative trait controlled by multiple interacting genetic factors: several quantitative trait loci, including qAftA07, qAftB06.2, qAFB1A07 and qRAF-14-1, have been consistently associated with reduced aflatoxin B1 and B2 accumulation. High-density SLAF-seq mapping further identified two stable QTLs, qRAF-3-1 and qRAF-14-1, containing disease and stress-related gene families, and candidate genes in these regions encode proteins involved in defense signaling, oxidative stress responses and secondary metabolism, including WRKY transcription factors, NLR proteins, lipoxygenases and cytochrome P450 enzymes.
Yet the review is emphatic that this genetic arsenal cannot work in isolation. The expression of genotypic resistance is highly influenced by storage and environmental conditions, reflecting genotype by environment by management interactions, meaning that genetic resistance alone cannot solve the problem unless combined with improved post-harvest management. Mechanical damage is a critical amplifier: cracks and abrasions caused during harvesting, shelling or handling compromise the protective seed coat, facilitate fungal entry and accelerate moisture uptake, and studies show that damaged kernels accumulate substantially higher aflatoxin levels than intact seeds under both field and storage conditions. Minimizing mechanical injury during post-harvest handling is therefore described as critical for reducing contamination, alongside the physical protection offered by intact seed coats and pods.
On the practical side, the review identifies drying and storage as the most important prevention methods. Drying post-harvest peanuts to safe moisture levels below 7 to 8 percent and using hermetic storage systems have been shown to reduce fungal growth in smallholder systems. Drying to an intermediate moisture level of 10 to 13 percent at harvest is considered sufficient to minimize mold proliferation before further curing to the safer storage threshold. Traditional sun drying, widely used in developing countries because of its low cost and simplicity, may extend beyond one week, whereas mechanical drying systems using heated air and controlled ventilation can reduce moisture to safe levels within 12 to 48 hours. In storage, high temperatures between 25 and 35 degrees Celsius, relative humidity above 70 percent and water activity greater than 0.85 are the main factors driving aflatoxin accumulation; one cited study found the maximum relative abundance of Aspergillus species in peanuts stored at 30 degrees Celsius and around 80 percent relative humidity, closely linked to higher aflatoxin levels in long-term trials. Hermetic packaging and modern storage structures that restrict moisture and oxygen are significantly better than traditional methods at reducing Aspergillus growth and toxin production.
The authors also outline breeding and biotechnology routes forward. Precision breeding combined with marker-assisted selection and genomic tools can introduce alleles that reduce Aspergillus infection and aflatoxin accumulation, while genome editing approaches such as CRISPR/Cas could accelerate improvement by precisely modifying genes controlling seed quality, resistance and post-harvest stability without introducing new DNA. Strengthening breeding programs with genetic markers alongside wild peanut germplasm, and developing climate-resilient and disease-resistant varieties, are presented as ways to lower fungal and pest pressure during storage and extend shelf life with reduced reliance on chemical controls. The review concludes that breeding strategies combining host resistance with improved post-harvest management practices offer sustainable reductions in aflatoxin risk.
Important limitations temper these conclusions. The authors state plainly that this is a narrative rather than systematic review, lacking formal screening, risk of bias assessment or quantitative pooling, so reported contamination ranges are illustrative rather than statistically synthesized. Most genotype-resistance studies cited were conducted under controlled or artificial inoculation conditions that may not fully reflect real-world storage variability, the search was limited to English-language sources within a specific time window, and differences in genotype, geography and measurement methods across studies limit direct comparison of reported figures. The review also flags substantial research gaps: molecular mechanisms underlying post-harvest resistance remain poorly understood, functional validation of candidate genes is still needed, genotype by environment by management interactions during storage are not well characterized, and fungal infection intensity does not always correlate with aflatoxin production, so direct toxin assessment is required. Priority research areas include standardized protocols for detecting pre- and post-harvest contamination, multi-location trials to evaluate the stability of genotype resistance, integration of direct toxin quantification with fungal infection studies, and affordable, climate-resilient post-harvest technologies suited to smallholder farming systems, where the review finds a persistent technology gap between commercial and smallholder operations.
Subject of Research: Post-harvest aflatoxin contamination in peanuts and integrated mitigation strategies
Article Title: Post-harvest aflatoxin contamination in peanut Arachis hypogaea mechanisms genotypic variation fungal ecology and mitigation strategies
Article References: Mequanint, G., & Wondmaneh, A. (2026). Post-harvest aflatoxin contamination in peanut Arachis hypogaea mechanisms genotypic variation fungal ecology and mitigation strategies. Discover Life, 56(1), Article 46. https://doi.org/10.1007/s11084-026-09765-1
Image Credits: AI Generated
DOI: 10.1007/s11084-026-09765-1
Keywords: aflatoxin, peanut, Aspergillus flavus, post-harvest management, genotypic resistance, food safety, hermetic storage, grain drying, quantitative trait loci, plant breeding, mycotoxins, storage conditions
News Source: Alan Morgan. (October 28, 2026). Resistant Peanut Varieties Alone Cannot Stop Aflatoxin, Review Finds. Scienmag.