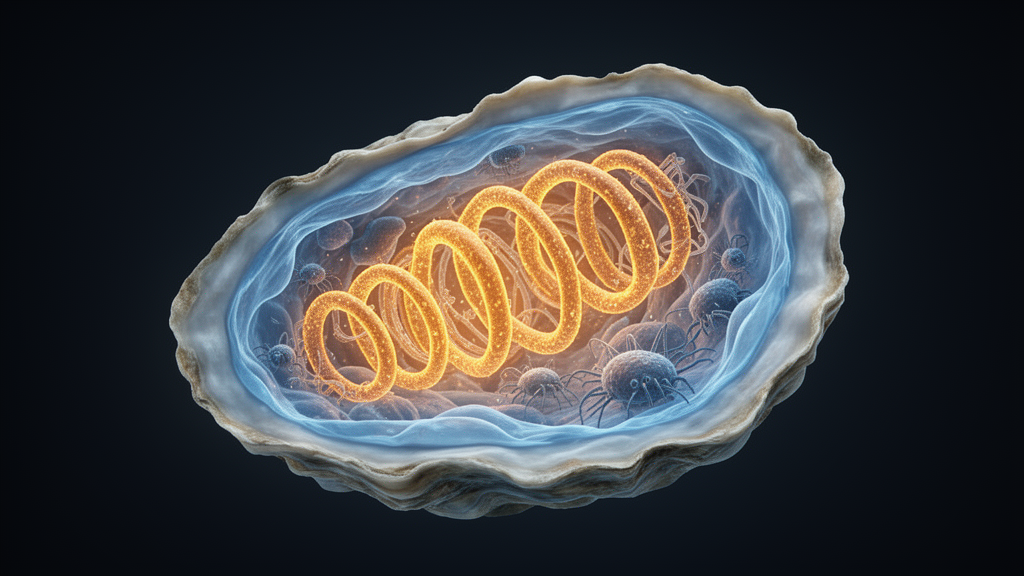
Deep beneath the surface of coastal waters, a single-celled parasite quietly attacks oyster populations, devastating aquaculture economies along the Atlantic and Gulf coasts of North America. That organism, Perkinsus marinus, the causative agent of Dermo disease, has now stepped into the scientific spotlight for an entirely different reason. A team of researchers led by Andrew E. Maclean and Lilach Sheiner, working alongside Julius Lukeš and colleagues, has used a sophisticated proteomic technique known as complexome profiling to map the molecular machinery inside the parasite’s mitochondria. Their findings, published in PLOS Pathogens, reveal that the strange, enlarged protein complexes that power the mitochondria of deadly apicomplexan parasites such as Plasmodium, the agent of malaria, and Toxoplasma gondii are not quirky evolutionary inventions of those pathogens. Instead, they are ancient features inherited from a common ancestor shared across an entire supergroup of single-celled eukaryotes known as the Myzozoa.
Mitochondria, the descendants of ancient bacteria that took up residence inside other cells more than a billion years ago, depend on a handful of large multiprotein assemblies to perform their essential duties. The mitochondrial electron transport chain, a series of respiratory complexes embedded in the inner membrane, shuttles electrons and pumps protons to generate the electrochemical gradient that drives the F1Fo-ATP synthase, the rotary molecular motor that manufactures most of the cell’s ATP. Alongside these energy-transducing machines sit the mitochondrial ribosome, or mitoribosome, which translates the handful of genes still encoded on the mitochondrial genome, and the Translocase of the Outer Membrane, or TOM complex, which imports the hundreds of proteins synthesized in the cytosol. In textbook animals and fungi, the compositions of these assemblies are well characterized and broadly similar. But over the past decade, studies of unicellular eukaryotes have exposed a startling degree of variation, with apicomplexan parasites emerging as particularly dramatic examples of divergence.
Apicomplexans, a group that includes the malaria parasites and Toxoplasma, have repeatedly remodeled their mitochondrial complexes, acquiring novel subunits that have no obvious counterparts in animals or plants. Some of these additions have been experimentally validated as essential for parasite growth, making them attractive candidates for drug development. What remained unresolved was whether these enlarged and divergent complexes were a recent innovation confined to the apicomplexan lineage, or whether they traced back to a deeper evolutionary origin. Answering that question required an organism positioned at a critical branching point in the eukaryotic tree of life, one close enough to apicomplexans to share their ancestry yet distinct enough to reveal which features are truly ancestral. Perkinsus marinus, a member of the Perkinsozoa, fits that role precisely.
The technique the researchers employed, complexome profiling, offers a powerful window into the native organization of protein assemblies within cells. Rather than analyzing proteins one by one after denaturing them, the method preserves intact complexes by gently solubilizing mitochondrial membranes, separates the assemblies according to their size under native conditions, and then slices the resulting separation profile into fractions. Each fraction is subjected to quantitative mass spectrometry, allowing every detected protein to be assigned a position along the size axis. Proteins that co-migrate in the same fractions across the profile are inferred to be components of the same complex, and shifts in migration relative to known markers can reveal changes in complex size or composition. Applied systematically, this approach produces a comprehensive map of the mitochondrial proteome organized by assembly, without requiring antibodies, genetic tags, or prior knowledge of each complex’s membership.
When Maclean, Iorillo, Faktorová, Singh, McGill, Lukeš and Sheiner applied this workflow to Perkinsus marinus, the results were striking. The parasite’s ATP synthase and electron transport chain complexes turned out to contain a suite of additional subunits previously identified only in apicomplexans. In Plasmodium and Toxoplasma, several of these components had already been shown through genetic studies to be important for parasite growth, underscoring their functional significance rather than mere decorative presence. Finding the same proteins assembled into the corresponding complexes in Perkinsus demonstrates that these subunits were present in the last common ancestor of the Myzozoa, the broader clade that unites apicomplexans, their closest relatives such as chromerid algae, the perkinsozoans, and the dinoflagellates. What had appeared to be a parasite-specific eccentricity is in fact a deeply conserved architectural plan.
Perhaps the most provocative discovery concerns the mitochondrial ribosome. Recent work on apicomplexans had revealed that their mitoribosomes carry a collection of divergent features, including associated proteins drawn from unexpected protein families. Among these are members of the ApiAP2 family, a group of proteins that, until those discoveries, had been considered exclusively as lineage-specific transcription factors regulating gene expression in the nucleus. The new complexome profile of Perkinsus shows that its mitoribosome possesses many of these same divergent characteristics, including ApiAP2 family members associated with the ribosomal assembly. The implication is remarkable: a protein family long defined by its role in DNA binding and transcriptional regulation has an ancestral, conserved second life inside the mitochondrial translation machinery of myzozoan organisms, a dual functionality that was invisible until proteomic methods capable of detecting native complexes were brought to bear.
The evolutionary logic of these findings carries weight beyond taxonomy. Myzozoans occupy a pivotal position in eukaryotic history, descending from photosynthetic ancestors through secondary endosymbiosis events and diversifying into lineages with radically different lifestyles, from free-living algae to obligate intracellular parasites. Establishing that the divergent mitochondrial complexes are shared across this breadth indicates that the remodeling occurred early, before the major myzozoan lineages split apart, and has since been maintained through hundreds of millions of years of evolution. Conservation on that scale suggests that the extra subunits are not evolutionary baggage but perform genuine, integrated roles, whether in stabilizing the complexes, regulating their activity, or mediating interactions unique to these organisms’ mitochondrial biology. For researchers studying mitochondrial evolution, Perkinsus now serves as a living fossil of sorts, preserving the ancestral myzozoan configuration of these molecular machines.
There are also practical consequences for human and animal health. Apicomplexan parasites impose an enormous burden on global health and agriculture, and the unusual subunits of their mitochondrial complexes have attracted attention precisely because they lack counterparts in their human or livestock hosts, offering the prospect of drugs that disable the parasite without harming the patient. A persistent concern in such efforts has been the possibility that each parasite lineage evolved its own idiosyncratic solutions, fragmenting the target space. The Perkinsus data counter that worry by showing that the divergent architecture is shared and conserved, which raises confidence that insights and inhibitors developed against one myzozoan mitochondrial complex may find relevance across the group. At the same time, the confirmation that essential growth factors in Plasmodium and Toxoplasma correspond to ancestral myzozoan components strengthens the case for these proteins as validated points of vulnerability.
Beyond the immediate findings, the study illustrates how much of eukaryotic molecular diversity remains hidden until the right lens is applied. Genome sequences alone could not have delivered these conclusions, because many of the divergent subunits are poorly conserved at the sequence level and their assignments to complexes depend on physical association rather than sequence similarity. Complexome profiling, by reading out the native assembly state of proteins, bridges that gap and can be deployed even in organisms that are genetically intractable, as many parasites and environmental protists are. As the method is extended across the tree of life, the picture emerging is one in which the mitochondrial complexes of model organisms represent only a narrow slice of a much richer evolutionary landscape. The oyster parasite, once studied chiefly as an economic threat to shellfish aquaculture, has now contributed a key piece to that broader map, anchoring the strange mitochondrial biology of malaria parasites to an ancient and enduring heritage shared across the Myzozoa.
Subject of Research: Mitochondrial complex composition in the myzozoan parasite Perkinsus marinus
Article Title: Complexome profiling of mitochondria in the myzozoan parasite of oysters, Perkinsus marinus
Article References: Maclean, A. E., Iorillo, O., Faktorová, D., Singh, M., McGill, S., Lukeš, J., & Sheiner, L. (2026). Complexome profiling of mitochondria in the myzozoan parasite of oysters, Perkinsus marinus. PLOS Pathogens, 22(9), e1014543. https://doi.org/10.1371/journal.ppat.1014543
Image Credits: AI Generated
DOI: 10.1371/journal.ppat.1014543
Keywords: Perkinsus marinus, mitochondria, complexome profiling, Myzozoa, apicomplexans, ATP synthase, electron transport chain, mitoribosome, ApiAP2, proteomics, PLOS Pathogens, parasite evolution
News Source: Gavin Prescott. (October 8, 2026). Oyster Parasite Reveals Ancient Blueprint of Divergent Mitochondrial Machinery. Scienmag.