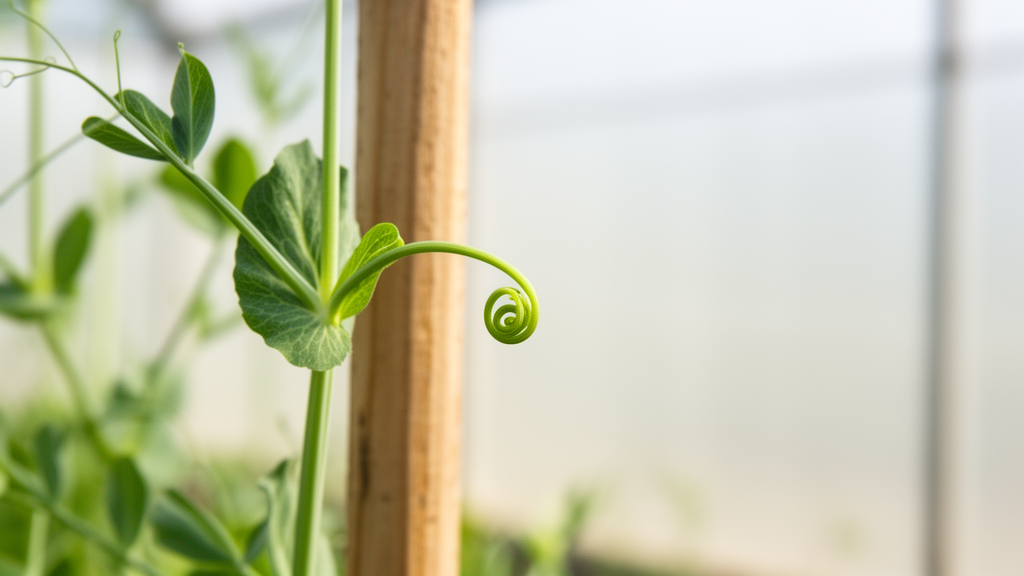
Climbing pea plants modulate the temporal dynamics of their approach-to-clasp movements when navigating external physical targets, demonstrating that environmental properties directly shape plant movement duration. In an experimental investigation published in Movement Ecology, researchers revealed that the time required for snow pea tendrils to reach and contact a support increases systematically as both the distance to the target and the width of the target increase. This observed pattern indicates that support distance and support thickness function as cumulative spatial constraints during plant search and attachment. These empirical findings demonstrate that reaching movements in plants do not follow a fixed developmental timeline, showing instead that organisms lacking a central nervous system systematically regulate their movement kinematics in response to external task demands.
In animal motor behavior, the relationship between movement duration and environmental task constraints is classically described by Fitts’s law, a principle establishing that movement time depends upon target distance and target width. Under the traditional animal framework, movement time increases as target distance increases but decreases when target width becomes wider, as broader targets provide larger landing zones that require less terminal precision. Mathematical formulations of Fitts’s law quantify task challenge via an Index of Difficulty defined by the logarithmic ratio of twice the distance divided by the width. Biologists have documented this predictive relationship across humans, non-human primates, rodents, and insects. However, climbing plants present a fundamentally distinct biological system because their reaching movements depend on growth, morphological development, and continuous oscillatory revolutions termed circumnutation. Because clasping a thicker pole requires substantial biological investment, researchers hypothesized that climbing plants would not conform to the classical inverse relationship with target width.
To test how spatial constraints regulate movement duration, the research team examined forty snow pea plants belonging to the cultivar Carouby de Maussane (Pisum sativum var. saccharatum). The study specifically evaluated successful approach-to-clasp behaviors across four controlled experimental treatments, assigning ten individual seedlings to each condition. Two wooden support widths were tested: a small pole measuring 1.1 centimeters in diameter and a large pole measuring 2.0 centimeters in diameter, each standing 60 centimeters tall and anchored 7 centimeters below the sand surface. These supports were positioned at two distinct horizontal distances: a near placement located 5 centimeters from the seedling origin and a far placement situated 10 centimeters away. These configurations formed four distinct experimental groups: small-near, small-far, large-near, and large-far, enabling direct evaluation of how target distance and support thickness independently and interactively influence movement kinematics.
All experimental trials were conducted within individual, strictly regulated growth boxes measuring 80 by 80 by 160 centimeters, maintained at a continuous ambient temperature of 26 degrees Celsius. Seedlings were germinated in darkness on absorbent paper following a 24-hour water soak, after which uniform specimens with comparable root and shoot lengths were transplanted into cylindrical pots filled with standardized silica sand. The plants received nutrient-rich liquid half-strength Murashige and Skoog basal salt micronutrient solution three times weekly. Illumination was provided by cool-white LED units positioned 50 centimeters above the pots on an 11-hour-15-minute light and 12-hour-45-minute dark photoperiod, synchronized with natural daylight to prevent circadian disruption. To eliminate directional phototropic cues and localized light reflection from the experimental posts, all internal chamber walls were completely lined with reflective Mylar film, and a specialized non-woven fabric template maintained precise planting distances across all experimental sessions.
Stereoscopic motion tracking captured the three-dimensional reaching trajectories without affixing physical reflective markers that could mechanically impede fragile plant tissues. Two high-resolution RGB-infrared cameras were positioned 110 centimeters above the floor and spaced 45 centimeters apart inside each growth box, synchronously acquiring image frames every three minutes at a frequency of 0.0056 Hertz. Contrast was maximized by lining internal walls with black felt velvet and coating the wooden poles with dark charcoal. Camera calibration and spatial depth reconstruction were achieved using an 18-millimeter square chessboard grid. Operators utilized specialized ROOMORS-TRACKING software, applying the Kanade-Lucas-Tomasi algorithm to follow virtual anatomical landmarks including the stem apex, the junction of the tendrils, and the distal tendril tips, while establishing fixed reference coordinates at the plant origin, second leaf, and support structures.
The primary kinematical dependent variable evaluated was movement time, defined as the duration in minutes elapsed between the initial visible emergence of tendrils from the apex and the exact frame showing initial tendril contact with the wooden pole. Kinematical analyses also quantified circumnutation parameters, tracking the total number of oscillatory cycles completed, the spatial trajectory length of each circumnutation in millimeters, and the individual circumnutation duration in minutes. At the conclusion of each trial, corresponding to the moment of initial support contact, researchers obtained precise morphological measurements. These physical metrics included total stem height measured across internodes with a caliper to 0.01-centimeter precision, the quantity of developed tendrils, individual tendril lengths, and primary root length determined with a millimeter-scale ruler after plant removal.
Statistical evaluation using linear mixed-effects models revealed that the classical formulation of Fitts’s law failed to explain pea plant movement duration. When testing movement time against the traditional Index of Difficulty, the relationship was positive but statistically non-significant (beta = 358.59, p = .154), yielding marginal and conditional coefficients of determination of 0.05 and 0.08, with growth box random variance accounting for only 2.7 percent of variation. Decomposing the classical index into independent spatial predictors revealed that movement time increased significantly with distance (log2 A: beta = 1179.0, p < .001) and increased significantly with target width (log2 W: beta = 774.6, p = .014). The statistical interaction between logarithmic distance and width was non-significant (beta = 761.7, p = .202), demonstrating that distance and support thickness operated as additive, cumulative constraints rather than opposing factors as seen in animal reaching tasks.
Because the empirical data demonstrated that broader supports lengthened rather than shortened movement duration, the investigators advanced an exploratory, plant-specific Index of Difficulty tailored to climbing organ mechanics. This modified mathematical formulation expressed task challenge through the logarithmic calculation ID_plant = log2((A * W) / k + 1), where A denotes distance, W represents width, and k reflects the product of average experimental distance and width. This normalization produced a dimensionless index reflecting relative environmental demands. When fitted in linear mixed-effects modeling, this plant-specific index demonstrated a highly significant positive relationship with movement time (beta = 2150.1, p < .001) and substantially improved statistical fit, dropping the Akaike Information Criterion from 677.0 under the classical model to 657.0, representing a Delta AIC of approximately 19.05, while reducing growth box random intercept variance to zero.
To evaluate whether movement time increases stemmed purely from physical growth requirements rather than behavioral modulation, the authors analyzed anatomical traits across experimental conditions. Although stem height differed across treatments (p = .007), with plants in the large-far condition reaching greater heights than those in the small-near condition, height and primary root length showed no correlation with one another (r = .002, p = .992). When experimental condition, stem height, and root length were simultaneously included in regression models predicting movement time, experimental condition remained a significant predictor (p = .008), whereas stem height (p = .307) and primary root length (p = .882) ceased to be significant. Similarly, while tendril count and tendril length varied across treatments, neither measure significantly predicted movement time when controlling for experimental condition, indicating that simple physical morphology cannot account for the temporal variations observed.
Instead, behavioral modulation was reflected in the dynamic structure of exploratory circumnutation movements executed prior to target contact. Modeling movement time against circumnutation kinematics demonstrated that the total count of circumnutations strongly predicted movement duration (F = 21.43, p < .001), whereas individual circumnutation length and mean duration were not significant predictors in that initial specification. Across conditions, plants exhibited significant variations in circumnutation duration (p < .001) and total circumnutation cycles (p = .011), with individuals facing the most challenging large-far condition executing significantly more circumnutations than those in the small-near group. When circumnutation dynamics were integrated into multi-variable models alongside experimental treatments, both circumnutation duration (p = .002) and cycle frequency (p = .008) significantly predicted movement time, demonstrating that climbing plants actively adjust their exploratory search patterns when encountering complex spatial demands.
These systemic behavioral adjustments highlight questions regarding how climbing plants detect support dimensions and coordinate shoot kinematics without specialized neural structures. Prior physiological research indicates that subterranean root systems play a critical role in sensing physical obstacles and environmental supports through mechanical touch sensing and exudate signaling. Mechanical stimulation of root tissues activates mechanosensitive calcium channels that generate rapid intracellular calcium waves propagating throughout vascular networks. In parallel, long-distance electrical potentials and the vascular transport of phytohormones including auxin, cytokinins, strigolactones, gibberellins, and abscisic acid facilitate coordinated communication between roots and aerial shoots. In the present study, roots consistently wound tightly around the buried portions of the wooden poles in all experimental conditions, corroborating prior findings that climbing pea plants integrate belowground tactile detection with aerial sensory inputs to calibrate clasping behavior.
The authors identified several methodological boundaries in their study, emphasizing that their plant-specific Index of Difficulty serves as a descriptive metric under the tested conditions rather than a universal physical law. Because observations ceased immediately upon initial tendril contact, the investigation did not evaluate subsequent stem coiling, structural anchorage, or potential trade-offs between reaching velocity and placement precision. Furthermore, the protocol evaluated only individuals that achieved successful attachment, precluding conclusions regarding how spatial constraints affect overall attachment probability. Evaluating only two discrete levels of distance and width constrained continuous functional modeling across broader ecological ranges. Nonetheless, the investigation provides definitive evidence that climbing plants systematically modulate movement duration in response to additive environmental constraints, expanding scientific understanding of biological movement regulation beyond neural organisms.
Subject of Research: Kinematic modulation of climbing pea plant movement under spatial task constraints
Article Title: Temporal dynamics of plant movement under task constraints
Article References: Guerra, S., Simonetti, V., Cannizzo, E., & Castiello, U. (2026). Temporal dynamics of plant movement under task constraints. Movement Ecology, 14(1), Article 67. https://doi.org/10.1186/s40462-026-00680-8
Image Credits: AI Generated
DOI: 10.1186/s40462-026-00680-8
Keywords: Pisum sativum, climbing plants, circumnutation, movement time, Fitts's law, spatial constraints, plant kinematics, plant behavior, root-shoot signaling, linear mixed-effects models, tendril movement, Index of Difficulty, 3D motion tracking, Movement Ecology, exploratory movement, mechanosensing
News Source: Drew Townsend. (November 20, 2026). Pea Plant Movement Time Increases with Support Distance and Pole Width. Scienmag.