An observational study comparing Caragana korshinskii plantations of different ages in China’s Mu Us Desert found persistent phosphorus limitation among soil microbes, with its modeled intensity lower in older stands. The space-for-time chronosequence included plantations established 10, 30, 50 and 70 years earlier and a mobile-sand-dune control. Extracellular-enzyme stoichiometry indicated that carbon limitation was strongest after the first decade and then broadly stabilized, while nitrogen limitation was not detected in the sampled plots. These results describe an association with stand age and restoration stage rather than a controlled demonstration of causation.
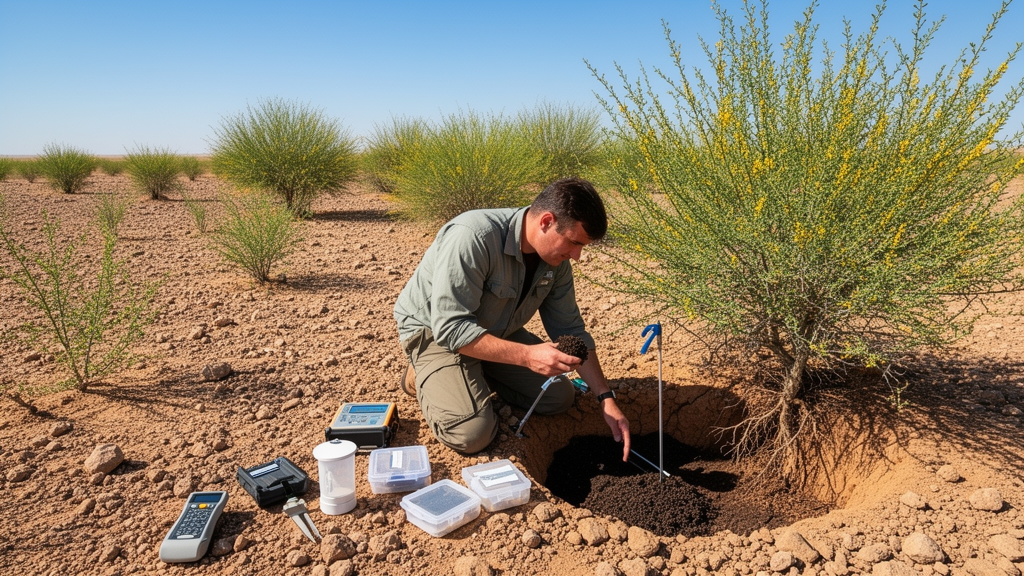
The fieldwork was conducted at the Baijiatan Nature Reserve on the southwestern edge of the Mu Us Desert in Ningxia, China. The site has a temperate continental semi-arid monsoon climate, with mean annual precipitation of 192.90 millimetres, potential evaporation of 1,933.3 millimetres and mean temperature of 8.8 degrees Celsius. Sandy soil predominates in an area that formerly consisted largely of mobile dunes with severe wind erosion and almost no surface vegetation. The researchers selected C. korshinskii stands established under similar initial soil, seedling and planting-density conditions. Three replicate 10-by-10-metre plots were established for each plantation age and for the control, with plots at least 100 metres apart, yielding 15 sampling plots.
Soil was sampled in August 2021, a period when plant growth and microbial activity were expected to be at their peak. Samples came from the upper 0–10 centimetres and were collected with five cores per plot, combined into one composite sample and passed through a sterile 2-millimetre sieve. Laboratory analyses quantified soil organic carbon, total nitrogen and total phosphorus, as well as microbial biomass carbon, nitrogen and phosphorus. Enzyme activities were measured by microplate fluorescence assays for β-1,4-glucosidase and cellobiohydrolase, representing carbon acquisition; β-1,4-N-acetylglucosaminidase and leucine aminopeptidase, representing nitrogen acquisition; and alkaline phosphatase, representing phosphorus acquisition. Activities were expressed as nanomoles per gram per hour.
The older plantations contained more of all three measured soil nutrients. In the 70-year-old stands, soil organic carbon averaged 14.08 grams per kilogram, total nitrogen 0.51 grams per kilogram and total phosphorus 0.15 grams per kilogram. The corresponding control-dune means were 1.43, 0.08 and 0.131 grams per kilogram. Soil carbon-to-nitrogen, carbon-to-phosphorus and nitrogen-to-phosphorus ratios generally increased across the chronosequence. Carbon-to-phosphorus rose from 10.864 in the control to 91.69 in the oldest stands, while carbon-to-nitrogen increased from 17.58 to 27.58 and nitrogen-to-phosphorus from 0.62 to 3.32. These unmatched increases show that the measured elements did not accumulate at the same rate across the plantation sequence.
Microbial biomass measurements followed a broadly similar age gradient. In the oldest stands, microbial biomass carbon, nitrogen and phosphorus averaged 72.80, 12.53 and 34.13 milligrams per kilogram, respectively, the highest values in the study. Microbial carbon-to-nitrogen and carbon-to-phosphorus ratios also reached their maxima in the 70-year-old stands, whereas the microbial nitrogen-to-phosphorus ratio did not change monotonically. These measurements describe the biomass pools’ elemental composition, not direct evidence that all microbial groups or ecosystem functions benefited equally. The study used microbial biomass composition together with extracellular-enzyme activity to infer the nutrient constraints facing the soil microbial community.
Activities of enzymes associated with acquiring carbon, nitrogen and phosphorus all increased through the plantation sequence and were significantly greater in the 70-year-old stands than in the younger plantations or the control. Their ratios followed more complex patterns. The enzyme carbon-to-nitrogen ratio peaked in the 10-year-old stand and then declined, while enzyme carbon-to-phosphorus also peaked at 10 years and subsequently stabilized. By contrast, the enzyme nitrogen-to-phosphorus ratio increased stepwise with stand age. Because resource-allocation theory links altered enzyme investment to microbial demand for limiting resources, these shifts were used in enzyme-stoichiometric models to estimate nutrient-use efficiency and the type and intensity of limitation.
The modeled carbon-use efficiency was highest in the mobile-dune control and lower at every plantation stage, with the 30-year-old stand recording the lowest estimate. Nitrogen-use efficiency increased substantially during the first 10 years and then tended to weaken, although the estimate for the 70-year-old stands remained above the control. The phosphorus-use-efficiency ranking was control, 10 years, 50 years, 70 years and 30 years. These are model-derived estimates based on enzyme ratios and stoichiometric inputs, not direct measurements of microbial growth or nutrient-use efficiency.
Enzyme-stoichiometric vector analysis distinguished the intensity of carbon limitation from the type of nitrogen or phosphorus limitation. In this model, vector length represents relative carbon limitation, while vector position relative to a 1:1 diagonal separates phosphorus from nitrogen limitation. All replicate plots across the control and four plantation ages were above that diagonal, indicating phosphorus limitation throughout the sampled chronosequence. The modeled degree of phosphorus limitation was strongest in the control and declined significantly across the sequence, with the 70-year-old stands showing the lowest value. Carbon limitation ranked from greatest to least as 10, 50, 70 and 30 years, with the control lowest. Relative carbon and phosphorus limitation were inversely associated, although that relationship alone does not establish a causal mechanism.
Multiple linear regression identified extracellular-enzyme carbon-to-phosphorus as the variable most strongly associated with the modeled limitation measures. For vector angle, a model retaining enzyme carbon-to-phosphorus, enzyme carbon-to-nitrogen and nitrogen-use efficiency explained more than 99 percent of the observed variation. For vector length, the retained variables were enzyme carbon-to-phosphorus, enzyme carbon-to-nitrogen, phosphorus-use efficiency and soil carbon-to-nitrogen; enzyme carbon-to-phosphorus again had the strongest association. These results came from only 15 plots, and the models retained only three or four predictors. Strong collinearity between enzyme carbon-to-phosphorus and enzyme nitrogen-to-phosphorus required one of them to be omitted, restricting conclusions about independent drivers.
The authors advance several non-mutually exclusive explanations for the persistent phosphorus limitation. As a nitrogen-fixing legume, C. korshinskii may provide continuing biologically available nitrogen through symbiotic rhizobia, potentially helping explain why nitrogen limitation did not emerge as microbial demand increased. In contrast, phosphorus input to desert soils depends largely on parent-material weathering and release from soil aggregates, and its conversion into available forms is comparatively slow. Greater microbial biomass and organic-matter accumulation in older stands may enhance organic-phosphorus mineralization, while expanded rhizospheres, root exudation and mycorrhizal associations may improve phosphorus acquisition. The study did not directly test these pathways, so they remain proposed mechanisms rather than demonstrated effects.
The chronosequence provides a detailed account of belowground changes across long-term desert restoration but cannot isolate shrub establishment as the cause of every observed difference. It compared different-aged plots rather than following the same plots through time, used 15 plots in total and did not comprehensively incorporate potentially influential environmental conditions such as soil moisture, temperature and pH. Enzyme activity can respond to those abiotic conditions as well as microbial demand. The findings therefore show that older C. korshinskii plantations were associated with higher nutrient stocks, altered enzyme stoichiometry and lower modeled phosphorus-limitation intensity, while early carbon limitation persisted. Direct phosphorus-addition experiments and additional measurements of physicochemical conditions would be required to test the proposed pathways and determine whether the pattern extends beyond C. korshinskii plantations in the Mu Us Desert.
Subject of Research: Extracellular-enzyme evidence of carbon, nitrogen and phosphorus limitation in soil microbes across Caragana korshinskii plantation ages in the Mu Us Desert
Article Title: Microbial nutrient limitations in soil during afforestation in the Mu Us Desert, China: insights from extracellular enzyme stoichiometry
Article References: Yu, S., Li, X., Norghauerf, J. M., Wang, X., Wan, Z., Yang, J., Yang, B., & Yang, H. (2026). Microbial nutrient limitations in soil during afforestation in the Mu Us Desert, China: insights from extracellular enzyme stoichiometry. Frontiers in Microbiology, 17, Article 1938090. https://doi.org/10.3389/fmicb.2026.1938090
Image Credits: AI Generated
DOI: 10.3389/fmicb.2026.1938090
Keywords: Mu Us Desert, Caragana korshinskii, microbial nutrient limitation, extracellular enzymes, ecological stoichiometry, phosphorus limitation, carbon limitation, nitrogen fixation, desert afforestation, chronosequence, Microbial, nutrient
News Source: Morgan Morrow. (October 21, 2026). Mu Us Desert Caragana chronosequence maps shifting microbial nutrient limitations. Scienmag.