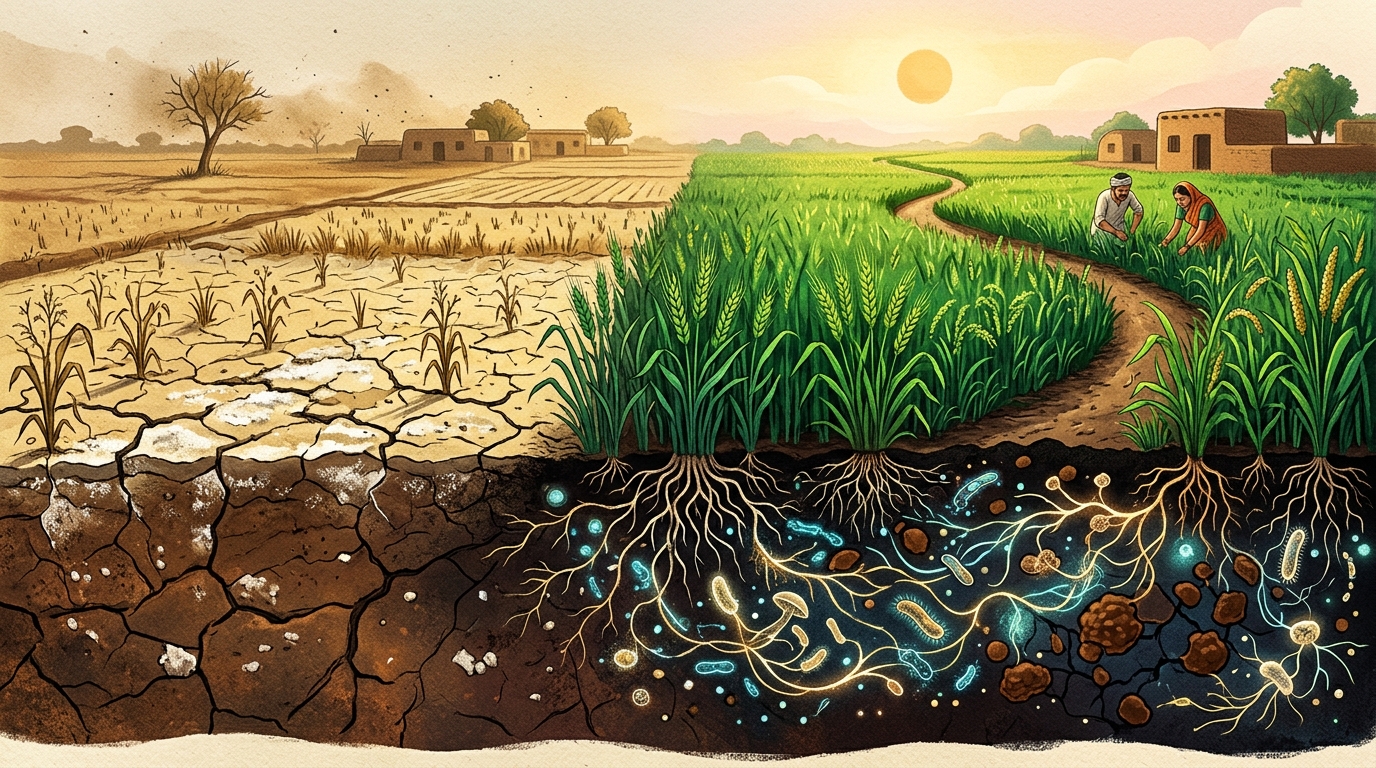
Degraded saline-alkali soils across semi-arid northwestern India severely limit ecosystem functioning and agroforestry productivity through elevated salinity, low organic carbon, restricted phosphorus availability and alkaline pH. A new field study reports that a carefully chosen set of organic-microbial amendments can shift several of these constraints within a single growing season, with measurable changes extending well below the layer where the materials were actually dug into the ground.
Researchers evaluated eleven amendment treatments built around two carrier materials: an enriched charcoal substrate, made from mixed-hardwood biochar pyrolysed at roughly 400 to 500 degrees Celsius and blended 1:1 with composted farmyard manure, and an enriched soil substrate, consisting of local agricultural topsoil mixed 1:1 with vermicompost. Each carrier was inoculated with one of four indigenous plant growth-promoting rhizobacteria, or with all four together, at 108 CFU per gram of substrate and incubated for seven days before field application. The bacterial strains were Klebsiella aerogenes, Lysinibacillus acetophenoni, Pseudomonas stutzeri and Pseudomonas mosselii, all isolated from nearby forest and agricultural soils and characterised for traits such as nitrogen fixation, phosphate solubilisation, indole-3-acetic acid production, siderophore synthesis and ACC-deaminase activity.
The trial was laid out as a randomised split-plot design at three research centres in Hisar, Karnal and Bhiwani districts, on soils classified as Inceptisols with alkaline pH, low organic carbon and limited nutrient availability. Each of the eleven post-treatment conditions, including an untreated control, was replicated in three plots per site, and every plot held 24 seedlings of Terminalia arjuna planted at 4 by 3 metre spacing. Importantly, the statistical unit was the plot, not the individual seedling, which guards against pseudoreplication. Soil samples were taken from each plot at three depth intervals, 0 to 30, 30 to 60 and 60 to 90 centimetres, with three subsamples per depth composited before laboratory analysis. Baseline measurements from untreated control plots, collected immediately before amendment application, served as site- and depth-specific reference values against which post-treatment changes were judged.
Electrical conductivity, the standard proxy for soil salinity, showed the most consistent response. Ten of the eleven amendments significantly reduced EC, and nine achieved significant reductions across all three depth intervals. The largest reductions reached 0.31 dS per metre at the surface, equal to 67 percent of the baseline value. At 0 to 30 centimetres, the strongest contrasts belonged to T2, enriched charcoal plus Klebsiella aerogenes, with an estimate of minus 0.309, T3, enriched charcoal plus Lysinibacillus acetophenoni, at minus 0.297, T11, enriched soil plus the four-strain consortium, at minus 0.294, and T7, enriched soil plus Klebsiella aerogenes, at minus 0.272, all with p values below 0.001. Effects were broadly maintained at 30 to 60 centimetres, where T2 and T3 again posted the largest reductions, and although attenuated at 60 to 90 centimetres, several treatments still showed significant EC declines, suggesting that salt amelioration extended into the subsoil despite the amendments being incorporated only into the upper 15 to 20 centimetres of soil.
Organic carbon responded in a strikingly depth-limited way. Eight treatments produced significant OC increases at 0 to 30 centimetres, with effect sizes of 83 to 109 percent above the site- and depth-specific baseline, in soils whose surface OC averaged 0.33 percent. The largest surface gains came from T7, enriched soil plus Klebsiella aerogenes, at plus 0.355, and T4, enriched charcoal plus Pseudomonas stutzeri, at plus 0.333. Yet no amendment produced a statistically significant OC increase at 30 to 60 centimetres, a pattern the authors attribute to the shallow incorporation depth and the inherent restriction of vertical particulate organic matter transport through undisturbed alkaline profiles. The single exception was T11, the enriched soil plus four-strain consortium, which produced a significant OC increase at 60 to 90 centimetres of plus 0.262 percent, with p equal to 0.014. The four-strain consortium encompasses biological nitrogen fixation, phosphate solubilisation, IAA production and ACC-deaminase activity, traits that may collectively stimulate root elongation, reduce salinity-induced ethylene stress and deepen root biomass allocation, although root distribution and microbial activity were not measured in the experiment, so this mechanism remains hypothetical.
Available phosphorus increased under multiple treatments at all three depths, a result the researchers interpret as consistent with microbial mobilisation of otherwise less-available phosphorus pools. In alkaline soils with pH between 7.85 and 8.05, phosphorus is predominantly fixed as calcium phosphates that are unavailable without active solubilisation, and the increases below the incorporation zone cannot be attributed solely to physical translocation of the solid amendment, suggesting that dissolved nutrient movement, rhizosphere processes or other within-profile processes may have contributed. The largest surface increases came from T5, enriched charcoal plus Pseudomonas mosselii, at plus 0.00159, and T2 at plus 0.00153, both with p values below 0.001. Significant phosphorus enrichment was also recorded at 30 to 60 centimetres for T2 and T3, and at 60 to 90 centimetres for several treatments. However, microbial abundance, enzyme activity and rhizosphere colonisation were not quantified, so the precise pathways cannot be confirmed from the present data.
Not every measured property moved. Soil pH, available nitrogen and available potassium showed no significant treatment effects during the study period, and the authors caution that the relatively short experimental duration may have limited the magnitude of detectable changes. The non-significant nitrogen result is particularly instructive. Nitrogen was the most depth-stratified variable in the analysis, with a depth main effect of F2,192 equal to 116.73 and p below 0.001, and the non-significant treatment effect indicates that nitrogen dynamics were governed by vertical gradients in biological activity rather than by these amendments during the study period. The authors propose several non-exclusive explanations for the absence of a nitrogen response, including possible microbial immobilisation of mineral nitrogen in the carbon-rich enriched charcoal, suppression of nitrogen fixation by ambient mineral nitrogen levels or restricted anaerobic microsites in these well-drained soils, and plant uptake by the transplanted seedlings offsetting any microbial fixation gains. Distinguishing these pathways would require measurements of microbial biomass nitrogen, nifH gene expression and plant tissue nitrogen that the present design did not include.
To synthesise the property-level responses into a composite measure, the team applied principal component analysis to six standardised soil properties and derived a Soil Quality Index weighted by the first principal component, which captured a dominant salinity-nutrient gradient. The first two components together explained 52.6 percent of total soil variability, with PC1 accounting for 28.6 percent and PC2 for 24.0 percent, reflecting the multivariate complexity of the data. On this index, T2, enriched charcoal plus Klebsiella aerogenes, recorded the highest overall mean SQI at 0.573, followed by T5, enriched charcoal plus Pseudomonas mosselii, at 0.396. T9, enriched soil plus Pseudomonas stutzeri, achieved the most depth-consistent profile, with a coefficient of variation across depths of just 26.1 percent and uniformly positive mean SQI values of 0.339, 0.249 and 0.203 at the three depth intervals. By contrast, T6, T7 and T8 produced near-zero overall SQI values (0.026, minus 0.014 and 0.013) with extreme depth variability (CV of 474 to 1119 percent), indicating that any surface-layer gains did not extend meaningfully into the subsoil, and depth-stratified assessment reveals treatment failures that surface-only designs would have misclassified as successes.
The statistical framework itself deserves attention. The team fitted separate linear mixed-effects models for each soil property using restricted maximum likelihood, with treatment, depth and their interaction as fixed effects and random intercepts for site and for plot nested within site and treatment. This structure ensures that inference rests on plot-level replication rather than inflated depth-level degrees of freedom. Marginal R2 values, representing variance explained by the fixed effects alone, ranged from 0.074 for potassium to 0.569 for nitrogen, while conditional R2 values, which add the hierarchical random-effects structure, ranged from 0.634 for EC to 0.881 for phosphorus among models with estimable conditional values. The gap between marginal and conditional values indicates that site- and plot-level heterogeneity accounted for substantial additional variation beyond treatment and depth, underscoring how strongly spatial structure shapes soil responses in this landscape. Between-site variance accounted for 58.6 percent of the observed variability in organic carbon and 56.4 percent in potassium, indicating substantial site-level heterogeneity, and OC improvements should be understood as the initiation of a multi-year trajectory rather than a step-change in soil organic matter status.
The authors are careful to frame their findings as treatment-associated changes under specific conditions rather than universal prescriptions. The experiment covered three sites and one post-treatment growing season, so the persistence of the observed responses, their economic feasibility and their broader applicability across the wider range of salt-affected soils remain uncertain. Mechanisms operating below the amendment incorporation layer, including salt redistribution, root-derived carbon inputs and microbial phosphorus solubilisation, remain plausible but unproven because the relevant processes were not measured directly. Within the conditions tested here, T2 and T5 warrant further field evaluation for their comparatively high composite soil quality, while T9 stands out for its depth-consistent performance. Multi-season experiments across additional sites, coupled with direct measurements of microbial processes, root dynamics, nutrient fluxes and amendment costs, are required before any of these combinations can be recommended for large-scale adoption.
Subject of Research: Microbial and organic amendments for reclaiming salt-affected semi-arid soils in northwestern India
Article Title: Reclamation of degraded saline-alkali soils of the northwestern region of India through microbial amendments
Article References: Kotiyal, P. B., Chauhan, V., Sharma, S. K., Soni, A., Kumar, M., Singh, R., Kumar, A., Kumar, D., Budhwal, R., Saini, V. K., & Rajjak, S. K. A. (2026). Reclamation of degraded saline-alkali soils of the northwestern region of India through microbial amendments. Discover Forests, 2(1), Article 86. https://doi.org/10.1007/s44415-026-00149-x
Image Credits: AI Generated
DOI: 10.1007/s44415-026-00149-x
Keywords: saline-alkali soils, soil reclamation, plant growth-promoting rhizobacteria, biochar, soil organic carbon, soil salinity, phosphorus availability, Haryana, Terminalia arjuna, soil quality index, mixed-effects models, Indo-Gangetic Plains
News Source: Alan Morgan. (November 4, 2026). Microbial amendments cut soil salt and lift carbon in degraded Haryana fields. Scienmag.