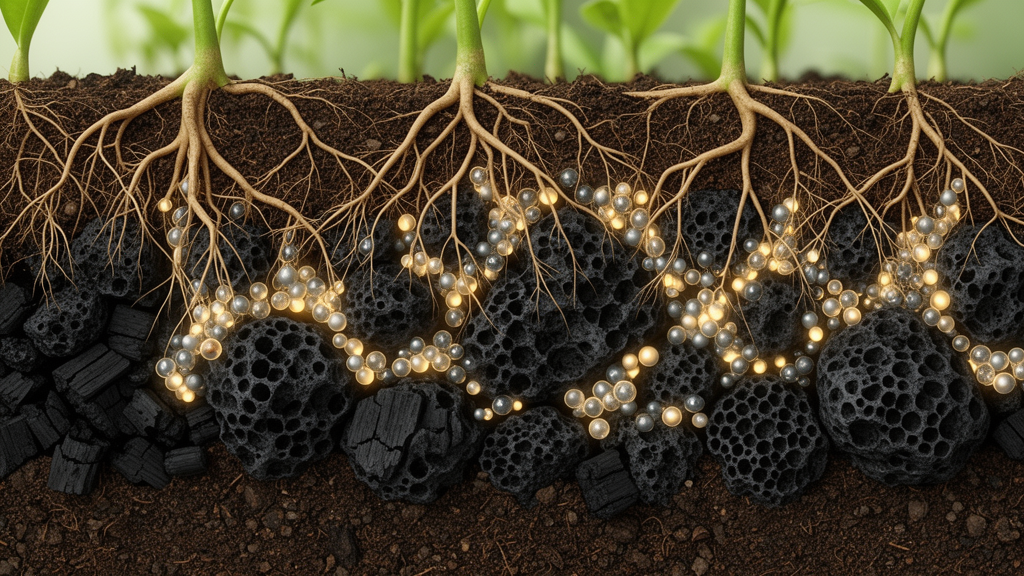
A comprehensive synthesis of soil and rhizosphere science demonstrates that biochar operates as an active interface engineer across the root–soil–microorganism continuum rather than functioning merely as an inert soil conditioner or bulk amendment. Across documented field and laboratory trials, biochar systematically modifies the physical, chemical, and biological gradients that define the millimeter-scale rhizosphere microdomain. In its physical role, biochar additions enhance soil aggregation by an average of 13.9% to 18.9% and elevate total porosity by 8.2% to 41.6%, relieving soil compaction and improving root elongation pathways. Chemically, the reactive functional groups, exchangeable base cations, and mineral ash components of biochar buffer rhizosphere acidity, alter localized redox equilibria, and coordinate sorption–desorption and complexation reactions. Biologically, the material supplies protected microhabitats that shelter bacteria and fungi from predatory protozoa and nematodes, while selectively enriching functional microbial taxa and stimulating metabolic activity. Across multiple ecosystems, these synchronized interfacial transformations elevate urease activity by an average of 23.1%, alkaline phosphatase by 25.4%, and the relative abundance of key nitrogen-cycling functional genes including amoA and nosZ by 25.3% and 17.0%, respectively.
The structural evolution of the rhizosphere physical framework under biochar amendment originates from the material’s internal porous architecture, large specific surface area, and abundant surface oxygen-containing functional groups. These properties facilitate strong organo-mineral binding between soil mineral grains, polyvalent cations, and native organic compounds, enabling biochar particles to serve as nucleation centers for macroaggregate formation. Concurrently, dissolved organic carbon released from biochar stimulates mycorrhizal fungi and rhizosphere microorganisms, producing hyphal networks and extracellular polymeric secretions that transform microaggregates into stable macroaggregates larger than two millimeters. Bulk density is typically reduced by 3% to 31%, with the most substantial decreases occurring in coarse-textured soils where looser matrices relieve the physical impedance encountered by expanding root tips. In addition to expanding total porosity, biochar alters pore size distributions by reducing the relative proportion of ultrafine pores and expanding larger, well-connected pore networks. This architectural reconfiguration substantially increases pore network continuity, enhancing oxygen diffusion toward roots, supporting aerobic respiration, and improving hydraulic conductivity, which in turn mitigates transient root hypoxia following precipitation or irrigation events.
Hydrological dynamics within the root zone respond non-linearly to biochar amendment based on soil texture, application rate, and particle dimensions. Global syntheses confirm that biochar improves plant-available water most substantially in coarse-textured substrates, producing increases of 45% to 51% in sand and loamy sand, approximately 20% in loam soils, and negligible shifts in heavy clay. This response reflects the infilling of wide interparticle voids with internal biochar micropores, which elevates the total volume of capillary pores capable of retaining water against gravity. In sandy loam soils under moisture deficits, biochar maintains continuous hydraulically conductive pathways, permitting transpiration rates to remain up to 83% higher than unamended controls. However, hydrological benefits depend strictly on rate and particle sizing: applications exceeding 30 to 60 tonnes per hectare or incorporating fine particles smaller than 0.5 millimeters can extend infiltration time and lower infiltration rates due to pore clogging and functional group water adsorption. While fresh unweathered biochar may temporarily impair water intake because of pyrogenic surface hydrophobicity, natural field weathering and surface oxidation progressively increase hydrophilicity, securing sustained improvements in rhizosphere water availability over multi-year periods.
At the chemical interface, biochar acts as a dynamic sorption reservoir and regulatory buffer governed by acid–base, complexation, and precipitation reactions. In acidic soils, alkaline minerals, carbonates, oxides, and hydroxides associated with biochar ash neutralize soil protons, providing acid-neutralizing capacity equivalent to up to one-third of agricultural lime. Pyrolysis temperature serves as the primary determinant of this liming capacity, as processing temperatures above 600 degrees Celsius eliminate acidic surface groups and enrich basic mineral ashes, generating alkaline biochar with pH values ranging between 5.43 and 10.8. Chemically, metal and nutrient immobilization occurs through distinct but overlapping pathways. Reversible ion exchange occurs at negatively charged surface sites, while stronger inner-sphere surface complexation forms stable coordination bonds between metal cations and surface carboxyl or phenolic hydroxyl groups. Concurrently, reactive phosphate and carbonate anions supplied by biochar precipitate sparingly soluble mineral phases such as cadmium and lead phosphates or carbonates. As biochar undergoes prolonged field aging, mineral ash components deplete while progressive surface oxidation generates new oxygen-containing functional groups, causing the dominant metal immobilization mechanism to shift over time from early ash-driven precipitation to sustained surface complexation and cation exchange.
Biochar also functions as an active participant in rhizosphere redox chemistry and electron transfer processes through its condensed aromatic carbon matrix, persistent free radicals, and reversible quinone–hydroquinone functional groups. These structural features allow biochar to serve as an electron donor, electron acceptor, or electron shuttle that accelerates microbial extracellular electron transfer across cell envelopes. This shuttling mechanism facilitates the dissimilatory reduction of insoluble iron(III) minerals to dissolved iron(II) and the reductive detoxification of mobile chromium(VI) to sparingly soluble chromium(III). Moreover, biochar establishes pronounced spatial redox heterogeneity within the root zone: enhanced pore connectivity promotes gas exchange to create oxic micro-zones, while internal water retention in micropores sustains localized anoxic microsites within the same structural aggregate. In flooded paddy soils, this dual microenvironment drives coupled iron, manganese, and sulfur redox cycling. Dissolved iron(II) generated in anoxic microsites migrates toward oxygenated root surfaces where radial oxygen loss oxidizes it into secondary iron plaque coatings, which sequester toxic cadmium and arsenic and prevent their translocation into edible crop tissues.
The biological re-engineering of the rhizosphere occurs through physical habitat creation, chemical niche differentiation, and metabolic regulation. Biochar contains a hierarchical pore network spanning macropores above 50 nanometers, mesopores between 2 and 50 nanometers, and micropores below 2 nanometers, which provide colonization surfaces and physical shelter from soil predators like protozoa. Over long-term applications, biochar enhances microbial network complexity by increasing node numbers, edge density, and clustering coefficients, while restructuring the functional backbone of the community through the enrichment of keystone taxa within Actinobacteriota, Proteobacteria, and Chloroflexi. At the metabolic level, biochar can enhance microbial carbon use efficiency by 11% to 39%, lowering metabolic maintenance energy requirements and shifting microbial community composition toward K-strategists. In long-term trials, this metabolic shift reduces the mineralization of native soil organic carbon by more than 5.5% on average through negative priming effects and organo-mineral microaggregate occlusion. However, microbial responses depend heavily on feedstock purity and pyrolysis conditions: low-temperature biochars produced between 350 and 400 degrees Celsius or amendments derived from sewage sludge and animal manures can introduce volatile organic compounds, heavy metals, or soluble potassium salts that temporarily inhibit sensitive taxa unless screened beforehand.
Biogeochemical cycles of key macro- and micronutrients are reshaped through these converging physical, chemical, and biological mechanisms. With respect to carbon cycling, recalcitrant aromatic carbon structures persist over centennial timescales, while optimized root penetration stimulates rhizodeposition, elevating root-derived carbon retention within stable subsoil fractions by an average of 20%. In the nitrogen cycle, biochar reduces nitrogen leaching by an average of 10.9% and inhibits ammonia volatilization via ammonium adsorption onto surface carboxyl groups and nitrification modulation, while alkaline biochar with carbon-to-nitrogen ratios exceeding 30 stimulates nosZ gene expression and suppresses nitrous oxide emissions by up to 76.7%. Phosphorus dynamics exhibit a sensitive bifurcation governed by soil pH: in acidic soils, biochar liming relieves iron- and aluminum-mediated phosphate fixation to increase plant-available orthophosphate, whereas high application rates in alkaline soils elevate calcium activity and induce calcium-phosphate precipitation, decreasing phosphorus flux by 11.6% to 79.0%. For essential cations, high-temperature biochars supply soluble potassium and retain calcium and magnesium, while silicon-rich feedstocks such as rice straw release monosilicic acid, promoting aluminosilicate formation and mitigating root aluminum toxicity.
Ecological functions at the whole-plant level are amplified through modulated rhizosphere signal transduction and stress mitigation pathways. Biochar adsorbs microbial signaling molecules, such as N-acyl homoserine lactones produced by Gram-negative bacteria, with high-temperature products altering quorum sensing and downregulating virulence in bacterial populations. Root exudate profiles are simultaneously modified, diminishing allelopathic phenolic acids and reducing root-knot nematode and Fusarium infestation. Concurrently, biochar triggers plant induced systemic resistance and systemic acquired resistance by upregulating defensive enzymatic cascades involving superoxide dismutase, peroxidase, catalase, and pathogenesis-related proteins. In response to abiotic stresses, biochar mitigates soil salinity by adsorbing sodium ions, supplying calcium and magnesium to displace exchangeable sodium, and upregulating plant ion transporter genes including SOS1 and NHX1 to sustain cellular potassium-to-sodium homeostasis. Under drought stress, enhanced water retention and the upregulation of plasma membrane intrinsic aquaporin genes stabilize plant water balance and preserve photosynthetic apparatus integrity.
Translating these mechanistic insights into agricultural and environmental management requires establishing quantitative dose-response thresholds tailored to specific soil contexts and evaluating full life cycle economic realities. Agronomic optimizations indicate that in alkaline sandy loam soils, coarse biochar derived from wood or crop residues produced above 500 degrees Celsius and sized between 0.5 and 2 millimeters yields optimal performance at rates of 20 to 40 tonnes per hectare, driving yield increases of 50% to 166%. Conversely, acidic sandy loams require lower application rates between 5 and 25 tonnes per hectare to prevent over-alkalization. Across economic evaluations, biochar systems face substantial cost hurdles: production expenses average 233 dollars per tonne, with feedstock acquisition accounting for up to 75% of costs, meaning commercial viability often demands monetization via carbon removal credits. In tropical settings such as Sub-Saharan Africa, sustained yield gains generate positive net present values over multi-decade horizons, whereas temperate European cropping scenarios often exhibit negative net present values without external financial incentives.
Deployment must also account for secondary environmental risks and unresolved scientific frontiers. During field weathering, physical, chemical, and biological fragmentation breaks bulk biochar down into mobile micro- and nano-scale colloids. Because chemical aging enriches negatively charged oxygen-containing functional groups and elevates zeta potential, aged nano-biochar exhibits high dispersion stability in soil pore water. Experimental column trials confirm that these mobile colloids compete with soil mineral surfaces and act as carriers, accelerating the downward co-transport of chromium(VI) by 0.5 to 7.0 times, while similarly mobilizing cadmium, phenanthrene, and atrazine toward underlying groundwater aquifers. Furthermore, feedstocks like sewage sludge introduce endogenous heavy metals and persistent free radicals that induce oxidative stress. The review concludes by outlining three research priorities: first, resolving context-dependent contradictions in hydraulic conductivity and phosphorus availability across varying soil textures and pH gradients; second, quantifying the decadal aging trajectories that govern when colloidal detachment risks outweigh surface complexation benefits; and third, deploying in situ millimeter-scale metatranscriptomics and enzyme assays to track dynamic rhizosphere microbial networks under real-world field conditions.
Subject of Research: Integrated physical, chemical, and biological mechanisms of biochar in the plant rhizosphere
Article Title: Biochar as a rhizosphere interface engineer: integrated regulation of microenvironments, biogeochemical cycling, and plant resilience
Article References: Gui, X., Zhao, Z., Zhang, Y., Zhou, D., He, J., Chu, C., Wang, Q., Hu, L., Li, F., Wu, S., & Cao, X. (2026). Biochar as a rhizosphere interface engineer: integrated regulation of microenvironments, biogeochemical cycling, and plant resilience. Biochar, 8(1), Article 135. https://doi.org/10.1007/s42773-026-00649-1
Image Credits: AI Generated
DOI: 10.1007/s42773-026-00649-1
Keywords: biochar, rhizosphere, soil aggregation, porosity, nutrient cycling, microbial ecology, extracellular electron transfer, carbon sequestration, nitrogen retention, phosphorus availability, iron plaque, abiotic stress, disease suppression, soil remediation, pyrolysis temperature, feedstock, nano-colloids, soil organic carbon
News Source: Morgan Morrow. (November 16, 2026). Biochar Reshapes Rhizosphere Microenvironments and Boosts Root Nutrient Retention. Scienmag.