Published in Heredity, the study evaluated more than a thousand single-nucleotide polymorphisms collected from eight natural populations distributed from sea level up to 2140 meters in altitude. The researchers found that despite pronounced ecophysiological contrasts between lowland and highland plants, elevational distance does not directly account for genetic differentiation across the landscape. Instead, the species is divided into two distinct genomic lineages that underwent early asymmetric gene exchange before becoming completely isolated during the Middle and Late Pleistocene, demonstrating how past climatic fluctuations shape montane biodiversity.
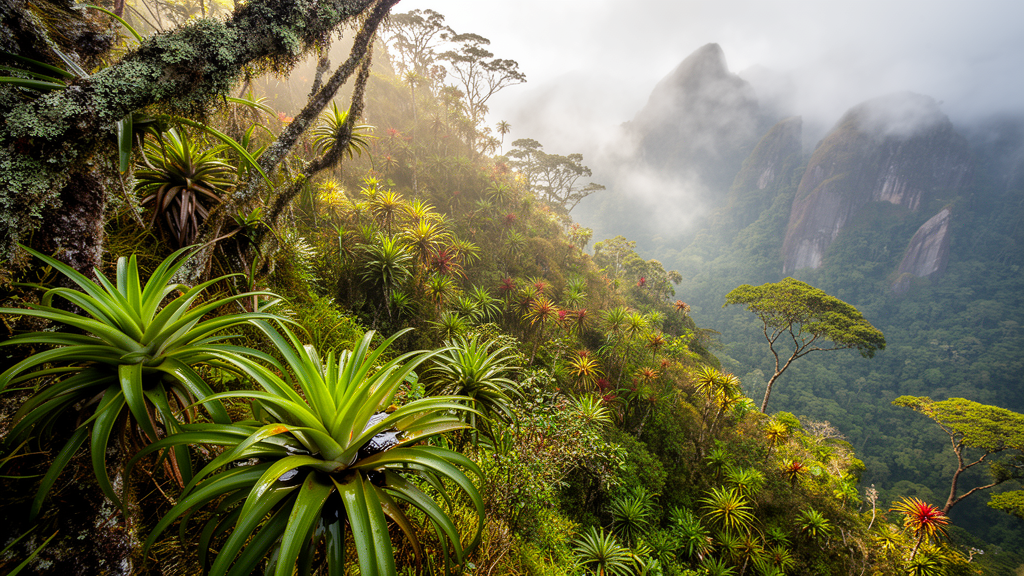
Montane elevational gradients have long served as natural laboratories for examining how environmental heterogeneity, geographic isolation, and historical climatic oscillations interact to generate biological diversity. The Brazilian Atlantic Forest represents an important Neotropical biodiversity hotspot characterized by naturally fragmented rocky habitats, steep topographic relief spanning up to 2900 meters above sea level, and pronounced environmental gradients. Pitcairnia flammea exhibits high morphological variability, restricted gene flow, and contrasting physiological strategies along altitudinal transects. This endemic bromeliad provides an exceptional model system for disentangling whether genetic differentiation across tropical mountains stems primarily from elevational adaptation or from historical climatic shifts and geographic isolation.
To minimize confounding spatial variation associated with latitude, collections were geographically restricted while spanning the entire elevational gradient. Total genomic DNA was extracted from fresh leaf tissue of 159 plants, averaging 20 individuals per locality, using a protocol combining sorbitol washings, cetyltrimethylammonium bromide extraction, and column isolation.
Restriction-site associated DNA sequencing was performed on an Illumina HiSeq 2000 platform using 150-base single-end reads following digestion with the restriction enzyme SbfI. Sequence reads were demultiplexed, filtered for quality, and aligned to the Pitcairnia flammea reference genome using the IPYRAD pipeline. To support distinct analytical requirements and prevent statistical biases, the researchers assembled four specialized genomic datasets. Dataset I comprised 1643 single-nucleotide polymorphisms selected as single markers per locus to reduce linkage disequilibrium. Dataset II retained 1560 loci after filtering for a maximum of 25 percent missing data and a minimum sequencing depth of 15. Dataset III assembled 12,356 biallelic markers without missing data across 40 individuals balanced between genetic groups. Dataset IV preserved between 18,203 and 28,599 loci across standardized subsets of ten individuals per population.
Because natural selection can distort demographic reconstructions, the researchers implemented two outlier detection methods to isolate putatively neutral loci for demographic modeling. Using Dataset I, the team applied principal components analysis in PCADAPT, which identifies outlier markers using Mahalanobis distances that measure significant deviations from population-wide allele frequency distributions. Concurrently, the Bayesian logistic regression framework in BayeScan was utilized to decompose locus-specific and population-specific differentiation components. These complementary analyses identified 174 outlier loci in PCADAPT and 32 outlier loci in BayeScan. All loci detected by either program were removed from Datasets III and IV. By systematically excluding loci under putative selection, the researchers ensured that subsequent inferences regarding historical effective population sizes, divergence times, and migration rates reflected neutral demographic processes and genetic drift.
Genetic diversity indices calculated in Stacks from Dataset II demonstrated that genetic variation was highest in the high-elevation populations. Pico dos Marins and Serra do Papagaio exhibited the greatest number of private alleles at 240 and 245, accompanied by polymorphic loci percentages of 19.30 percent and 18.10 percent, elevated nucleotide diversity values of 0.042 and 0.040, and expected heterozygosities of 0.041 and 0.043. Observed heterozygosity was similarly elevated at 0.042 in Marins and 0.039 in Papagaio. The intermediate-elevation population of Maria Comprida showed diversity patterns comparable to the high-elevation summits. Inbreeding coefficients remained low across all eight populations, showing even lower values at higher elevations, ranging from 0.003 at Pedra do Sino and 0.010 at Pico dos Marins to 0.011 at Itatiaia and 0.015 at Serra do Papagaio.
Multivariate and model-based clustering analyses revealed pronounced genetic structure among the sampled localities. Bayesian clustering in STRUCTURE identified two primary genetic clusters under the delta K criterion. Group 1 joined the high-elevation populations of Pico dos Marins and Serra do Papagaio with intermediate-elevation Maria Comprida, while Group 2 encompassed low- and mid-elevation populations from Pedra do Sino, Itatiaia, Corcovado, Morro do Rangel, and Ubatuba. Discriminant analysis of principal components further separated Maria Comprida and distinguished Marins from Papagaio across four clusters. Maximum likelihood clustering in ADMIXTURE resolved each geographic population into a distinct cluster, except for the geographically proximate lowland sites of Morro do Rangel and Corcovado. A neighbor-joining network in SplitsTree5 corroborated these divisions, showing that each rock outcrop acts as an independent genetic unit.
To assess whether geographic distance or elevational divergence governed genetic differentiation, the team performed Mantel and partial Mantel tests on linearized fixation indices. Pairwise fixation values confirmed substantial divergence between highland and lowland groups, but Mantel tests showed no significant correlation between geographic distance and genetic differentiation, producing a correlation coefficient of 0.022 and a p-value of 0.415. Similarly, isolation-by-elevation tests revealed no significant relationship between elevational distance and genetic divergence, yielding a correlation of 0.256 and a p-value of 0.086. When partial Mantel tests controlled for geographic distance, the correlation remained non-significant at 0.257 with a p-value of 0.091. Spatial modeling in Estimated Effective Migration Surfaces confirmed that contemporary gene flow is highly restricted, demonstrating that genetic divergence is not driven by altitudinal distance alone.
Phylogenetic population tree inference in SNAPP using 1560 single-nucleotide polymorphisms resolved four main evolutionary branches and clarified lineage divergence times. Calibrating the tree with a plant mutation rate of 3.0 multiplied by ten to the negative ninth substitutions per site per generation and a five-year generation time, the analysis dated the initial divergence between high-elevation populations and lower-elevation groups to approximately 275,000 years ago, with a 95 percent highest posterior density interval of 226,000 to 325,000 years ago. High-elevation lineages Marins and Papagaio split from each other around 150,000 years ago, whereas lower-elevation populations diversified around 60,000 years ago. Maria Comprida diverged from the Group 2 ancestral lineage approximately 250,000 years ago, despite its clustering affinity with Group 1, highlighting complex evolutionary relationships dating to the Middle and Late Pleistocene.
Demographic modeling using FASTSIMCOAL evaluated four alternative historical gene flow scenarios between the two primary genetic groups. Coalescent simulations based on the joint site frequency spectrum decisively supported an early gene flow model over scenarios of complete isolation, continuous migration, or secondary contact, producing an Akaike Information Criterion value of 55,035.09 and a delta AIC difference of 71.65 over the second-best model. Parameter estimation indicated that gene flow between the groups ceased approximately 67,000 years ago. Migration was markedly asymmetric, with gene movement from Group 2 into Group 1 estimated at 7.3 multiplied by ten to the negative fifth, compared to 1.3 multiplied by ten to the negative sixth in the opposite direction. This directional gene flow likely contributed to the elevated genetic diversity observed in highland populations.
Historical changes in effective population size were reconstructed using FASTSIMCOAL modeling and non-parametric STAIRWAY PLOT 2 analyses based on folded site frequency spectra. FASTSIMCOAL identified population size contractions as the best-supported model for Marins, Itatiaia, Ubatuba, Papagaio, and the combined Rangel-Corcovado cluster, whereas expansions were supported for Pedra do Sino and Maria Comprida. STAIRWAY PLOT 2 demonstrated that effective population sizes fluctuated throughout the Pleistocene, with several populations exhibiting declines within the last 100,000 years. Pico dos Marins expanded around 750,000 years ago before stabilizing and experiencing a slight decrease over the past 20,000 years. Pedra do Sino underwent a pronounced contraction after 20,000 years ago, coinciding with the Last Glacial Maximum, while Maria Comprida increased between 300,000 and 150,000 years ago before declining and stabilizing near 50,000 years ago.
These genomic and demographic results are consistent with the flickering connectivity hypothesis, which explains how Pleistocene climate oscillations periodically altered habitat connectivity across tropical mountains. During cold, humid glacial periods, vegetation shifted downslope, establishing temporary corridors that permitted episodic gene exchange between fragmented rock outcrop populations. Subsequent warm, dry interglacial stages caused habitats to contract upslope, severing connectivity and promoting genetic drift. Previous physiological studies demonstrated that high-elevation Pitcairnia flammea plants rely on cold and heat tolerance, whereas lowland populations rely on water-saving strategies. The present genomic findings indicate that these physiological distinctions parallel historical divergence, showing that Atlantic Forest montane diversity reflects the combined effects of Pleistocene climatic oscillations, topographic complexity, and restricted connectivity.
Subject of Research: Population genomics and demographic history of Pitcairnia flammea across an elevational gradient in the Brazilian Atlantic Forest
Article Title: Population genomic differentiation and demographic history across an elevational gradient in an endemic bromeliad of the Atlantic Forest mountains
Article References: Cacossi, T. D. C., Chaves, C. J. N., Tavares, M. M., Aecyo, P., Leal, B. S. S., da Silva, R., Pinheiro, F., Sanín, M. J., & Palma-Silva, C. (2026). Population genomic differentiation and demographic history across an elevational gradient in an endemic bromeliad of the Atlantic Forest mountains. Heredity. https://doi.org/10.1038/s41437-026-00903-z
Image Credits: AI Generated
DOI: 10.1038/s41437-026-00903-z
Keywords: Pitcairnia flammea, Bromeliaceae, Brazilian Atlantic Forest, population genomics, elevational gradient, Pleistocene climatic oscillations, flickering connectivity hypothesis, restriction-site associated DNA sequencing, FASTSIMCOAL, SNAPP, STAIRWAY PLOT 2, isolation by elevation, isolation by distance, effective population size, asymmetric gene flow, inselbergs, sky islands, genetic diversity
News Source: Juliet Wilcox. (November 14, 2026). Pleistocene Climate Shifts Shaped Atlantic Forest Bromeliad Divergence Over Elevation. Scienmag.