A 65-day controlled incubation study using stable isotope tracing has revealed that amendments of rice straw and straw-derived biochar stimulate fundamentally different microbial ecological strategies to regulate soil organic carbon storage in paddy soils. Soils represent the largest terrestrial carbon pool, storing approximately 2400 gigatons of carbon within the upper two-meter depth globally, and an annual increase of four parts per thousand in soil organic carbon stocks could theoretically offset approximately 30 percent of global greenhouse gas emissions. Accumulation of organic carbon in soil environments depends upon the dynamic balance between two distinct functional fractions: particulate organic carbon, which represents a relatively labile pool derived primarily from partially decomposed plant fragments undergoing rapid turnover, and mineral-associated organic carbon, which is largely formed from microbial metabolites and cellular residues stabilized via interactions with mineral components. While earlier research established that exogenous organic inputs influence carbon stocks, the exact mechanisms by which substrate energy quality filters microbial life-history traits to regulate these distinct fractions in paddy agroecosystems have remained incompletely understood.
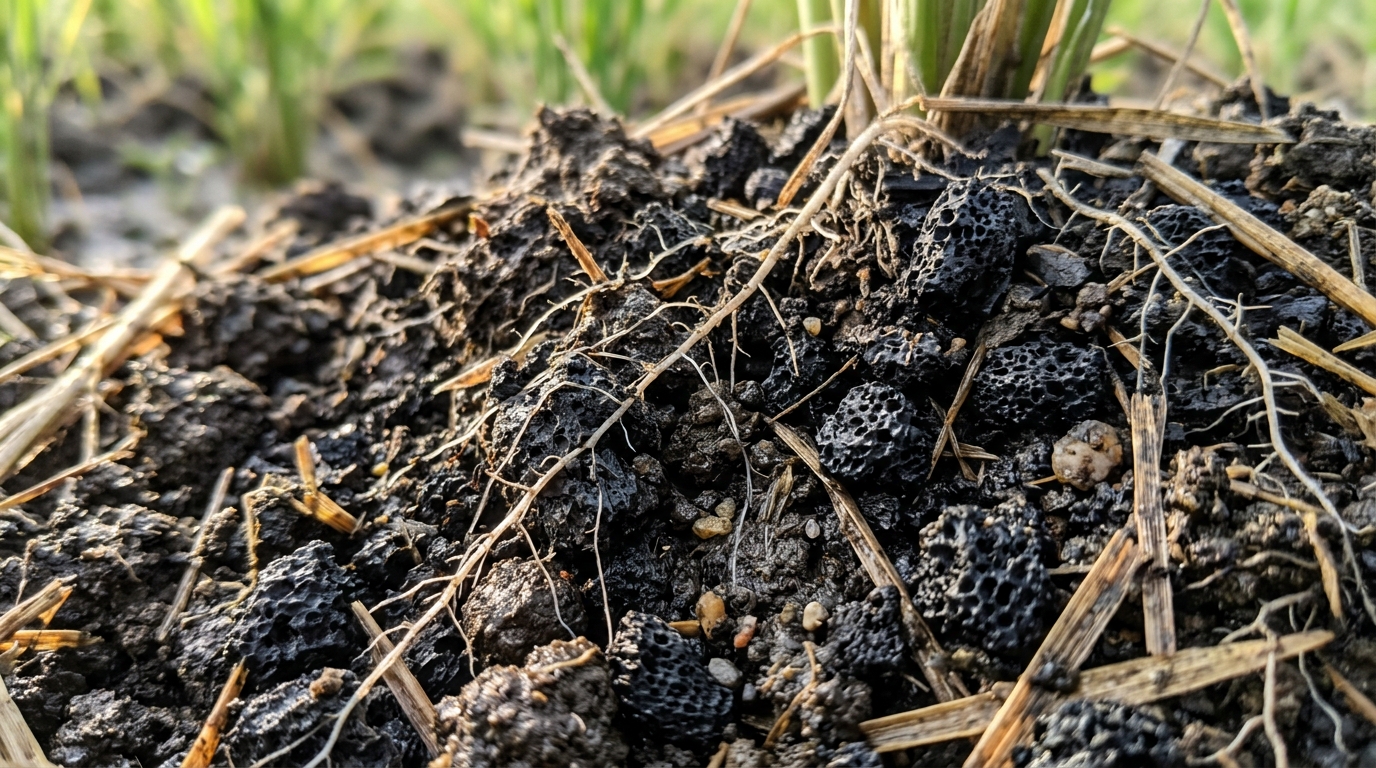
To systematically untangle the complex interactions among carbon inputs, microbial life-history strategies, and organic matter stabilization pathways, the research team conducted a laboratory incubation using topsoil collected from a long-term rice-rape cropping rotation established since 2011 at the Yangdu Research Station of the Zhejiang Academy of Agricultural Sciences in Jiaxing City, Zhejiang Province. Paddy soil gathered from the zero to twenty centimeter layer was homogenized, air-dried, and sieved through a two-millimeter mesh following a five-point sampling design across a ten-meter by ten-meter field plot. Stable carbon-13 isotope pulse labeling was conducted inside a closed plexiglass chamber using barium carbonate powder and hydrochloric acid under monitored carbon dioxide levels to generate uniformly labeled rice straw. A portion of this labeled straw was then pyrolyzed under oxygen-limited conditions at a heating rate of five degrees Celsius per minute up to a peak temperature of 500 degrees Celsius and held for two hours to synthesize labeled biochar. Before initiating the formal experiment, soil samples were pre-incubated for seven days at 40 percent field water-holding capacity to stabilize indigenous microbial populations, after which 100 grams of soil was thoroughly combined with either straw or biochar at an application rate of four grams of carbon per kilogram of soil alongside unamended control treatments maintained at 60 percent water-holding capacity at 25 degrees Celsius.
Over the course of the 65-day trial, the researchers observed marked contrasts in carbon fraction dynamics and overall sequestration between the two organic amendments. Measurements taken on the tenth day showed that straw amendment increased particulate organic carbon by 64.7 percent, mineral-associated organic carbon by 17.0 percent, and total soil organic carbon by 46.7 percent compared to the control, whereas biochar addition increased particulate organic carbon by 119 percent, mineral-associated organic carbon by 5.78 percent, and total soil organic carbon by 77.0 percent. By the sixty-fifth day, particulate organic carbon, mineral-associated organic carbon, and total organic carbon under straw amendment were elevated by 58.9 percent, 13.3 percent, and 38.7 percent, respectively, relative to control soils. In sharp contrast, biochar-amended soils exhibited increases of 174 percent in particulate organic carbon, 11.9 percent in mineral-associated organic carbon, and 103 percent in total organic carbon at day 65. The particulate organic carbon pool under biochar treatment was composed of both biochar-derived carbon and native soil-derived carbon, pointing toward physical retention and the aggregation of native organic matter alongside the recalcitrant added material.
Isotopic tracing through 21 periodic headspace gas samplings analyzed via isotope ratio mass spectrometry paired with gas chromatography highlighted stark divergences in microbial respiration and priming effects on native soil organic matter. Straw amendment generated substantially higher cumulative emissions of total carbon dioxide, carbon-13 dioxide, and carbon-12 dioxide compared to biochar, inducing an intense positive priming effect that accelerated the decomposition of indigenous soil carbon stocks. The researchers observed that the high-energy, readily available carbon provided by straw stimulated microbial nitrogen mining, causing microbes to mineralize native organic matter to satisfy their nutrient requirements. Consequently, the net carbon balance and sequestration efficiency of the straw treatment declined steeply over time, falling from a sequestration efficiency of 55.7 percent on day 10 down to just 22.8 percent on day 65. Conversely, biochar addition induced a negative priming effect that suppressed native carbon mineralization, yielding a stable net carbon balance that was 79.9 percent higher at day 10 and 338 percent higher at day 65 than that of straw, ultimately achieving an end-of-incubation carbon sequestration efficiency of 99.7 percent.
The pronounced differences in carbon retention were directly reflected in soil biochemical properties and hydrolytic enzyme dynamics. Straw incorporation significantly raised dissolved organic carbon by 19.5 to 40.8 percent and microbial biomass carbon by 124 to 155 percent throughout the incubation, accompanied by an initial 590 percent surge in microbial biomass nitrogen at day 10 that subsequently dropped by 74.2 percent at day 65. Straw also dramatically accelerated the activities of multiple extracellular enzymes, including beta-glucosidase by 337 to 416 percent, beta-1,4-N-acetylglucosaminidase by 158 to 449 percent, leucine aminopeptidase by 37.3 to 92.9 percent, and acid phosphatase by 68.7 to 140 percent. These elevated enzyme activities and accompanying vector metric shifts demonstrated enhanced microbial investment in acquiring carbon and alleviating nutrient limitations. Biochar amendment, while also elevating soil pH from 5.10 to 8.66 percent and ammonium nitrogen by 68.6 to 324 percent, reduced acid phosphatase activity by 11.3 percent at day 10 and suppressed beta-1,4-N-acetylglucosaminidase activity by 26.2 percent at day 65, reflecting reduced biological nitrogen mining and an adsorption-mediated limitation of enzyme-substrate interactions.
High-throughput sequencing of bacterial 16S ribosomal RNA genes and fungal internal transcribed spacer regions on the PacBio Sequel IIe platform confirmed that the two amendments favored distinct microbial life-history classifications. In the straw-treated soils, the influx of labile carbon stimulated copiotrophic r-strategist taxa, including the fungal phylum Mortierellomycota and the bacterial phylum Firmicutes, while significantly lowering bacterial Chao richness and Shannon diversity indices due to competitive exclusion by fast-growing organisms. By contrast, biochar created a stable microhabitat without inducing severe community diversity declines or major compositional shifts relative to the control, yet it distinctly enhanced the relative abundances of oligotrophic K-strategist microorganisms, such as the bacterial phyla Actinobacteriota and Chloroflexi as well as Basidiomycota, relative to the straw-amended soils by day 65. Principal component analysis and PERMANOVA tests verified that both bacterial and fungal community structures separated cleanly across treatment groups by the end of the incubation.
Analysis of soil amino sugar biomarkers—including muramic acid, mannosamine, galactosamine, and glucosamine quantified through ultra-performance liquid chromatography coupled to high-resolution mass spectrometry—demonstrated divergent pathways of microbial necromass accumulation. By the end of the experiment, straw amendment increased muramic acid and bacterial necromass carbon by 95.5 percent, fungal necromass carbon by 25.4 percent, and total microbial necromass carbon by 39.5 percent over the control. Biochar amendment yielded more selective changes, significantly increasing muramic acid, mannosamine, galactosamine, and bacterial necromass carbon by 37.3 percent, 14.2 percent, 32.2 percent, and 37.3 percent, respectively, but exerting no statistically significant effect on glucosamine, fungal necromass carbon, or total microbial necromass carbon. These biomarker patterns indicate that both amendments foster mineral-associated organic matter formation via bacterial cellular residue stabilization, while straw uniquely stimulates fungal residue accumulation.
Statistical modeling through random forest algorithms and structural equation modeling further detailed the direct and indirect causal pathways governing organic carbon fraction dynamics under each amendment. In the straw model, which explained 89 percent of the variance in total soil organic carbon, dissolved organic carbon served as the primary driver, exercising total path coefficients of 0.78 on particulate organic carbon, 0.84 on mineral-associated organic carbon, and 0.85 on total organic carbon. Specifically, dissolved organic carbon promoted particulate organic carbon directly and indirectly through acid phosphatase and Mortierellomycota abundance, while fostering mineral-associated organic carbon accumulation via beta-1,4-N-acetylglucosaminidase and Firmicutes. Under biochar amendment, structural equation modeling accounted for 91 percent of total organic carbon variance, with particulate organic carbon showing direct positive dependencies on dissolved organic carbon and microbial biomass carbon. Mineral-associated organic carbon accumulation under biochar was governed by a dual regulatory mechanism: microbial biomass carbon and leucine aminopeptidase activity exerted negative direct path coefficients of minus 0.22 and minus 0.61, whereas dissolved organic carbon, Actinobacteriota, and Chloroflexi contributed positive path coefficients of 0.49, 0.50, and 0.50, respectively.
Synthesizing these findings, the authors highlighted that the two management inputs mediate carbon stabilization through distinct biological and physical mechanisms that carry contrasting tradeoffs for long-term sequestration. Straw provides readily decomposable carbon that feeds fast-growing r-strategists, driving particulate organic carbon accumulation through hyphal fungal networks and mineral-associated carbon through rapid bacterial turnover; however, its low microbial carbon use efficiency and strong positive priming effect cause extensive native carbon loss, restricting overall sequestration efficiency. In contrast, biochar physically protects organic matter through its porous, recalcitrant structure and aggregate binding, suppresses enzymatic breakdown, and directs slow-growing K-strategist bacteria toward the high-efficiency synthesis of stable microbial necromass. The authors caution that the 65-day laboratory trial represents a brief experimental timeframe relative to biochar’s estimated multi-century residence time in soils, noting that field validation across decadal scales and higher-resolution temporal sampling between days 10 and 40 will be essential to evaluate whether combined applications of straw and biochar can concurrently optimize multiple carbon sequestration mechanisms in agricultural soils.
Subject of Research: Microbial life-history strategies and soil organic carbon sequestration under straw and biochar amendments
Article Title: Microbial life-history strategies mediate differential effects of straw and biochar amendments on soil POC/MAOC dynamics and SOC sequestration
Article References: Na, L., Liu, Y., Nan, Q., Chen, L., Dong, D., Wu, W., Tang, J., Yang, S., & Liu, Y. (2026). Microbial life-history strategies mediate differential effects of straw and biochar amendments on soil POC/MAOC dynamics and SOC sequestration. Biochar, 8(1), Article 118. https://doi.org/10.1007/s42773-026-00630-y
Image Credits: AI Generated
DOI: 10.1007/s42773-026-00630-y
Keywords: soil organic carbon, biochar, rice straw, microbial ecology, carbon sequestration, particulate organic carbon, mineral-associated organic carbon, priming effect, paddy soils, amino sugar biomarkers, Microbial, life-history
News Source: Alan Morgan. (November 7, 2026). Biochar and Rice Straw Drive Distinct Microbial Pathways for Soil Carbon Sequestration. Scienmag.